Chapter 3
Notes, Beats and Patterns: Three Anthropomimetic Features of Musical Lines
Abstract
Of the innumerable ways in which music can be constructed and appreciated, three features stand out as defining characteristics. First, music tends to utilize pitched tones. Second, music often is organized around regular beats. Third, music is constructed using recognizable patterns. It is argued from psychological and neurological evidence that these three musical features are explicitly anthropomimetic, causing musical sounds to be especially compelling and capable of expressing human emotion. Importantly, all three of these features are present in musical lines.
If music exhibits auditory animacy cues, it joins a broad category of percepts including barking dogs, revving engines, and trotting horses. But among a diverse array of apparently animate sounds encountered daily, music seems to be particularly expressive and emotionally compelling. It will be seen that music’s peculiar ability to captivate us could be attributed to its anthropomimesis. In other words, not only is music created by humans, but it also specifically resembles basic human features.
Percepts of a Social Animal
There are few creatures on the planet as social as human beings, we who rely on relationships with other people to fulfill innumerable short-term and long-term needs. Other people are our friends and loved ones, those with whom we build communities and on whom we rely for support. Other humans are also authority figures, teachers, teammates, or rivals. Each of us relies on a network of social alliances to help us navigate the densely populated world we inhabit. The human impulse toward interpersonal interaction is so strong that depriving somebody of human contact is among the most torturous of punishments, and chronic depression is often nearly indistinguishable from chronic loneliness (Cacioppo & Patrick, 2008).
This overwhelming human fascination with other humans is abundantly evident in the art and media we produce. Flipping through television or radio stations, one finds human likeness in sound or image practically inescapable. Even when nonhuman landscapes or structures appear onscreen, they are almost invariably accompanied by the sound of human narration. One would no more expect to find a motionless piece of furniture televised than grass growing or paint drying. Literature proves to be no different; fictional works concern humans and their affairs, and even if actual human animals never appear, anthropomorphized animals or objects are ready surrogates. In many ways, the world we inhabit is constructed by and of human beings and their relationships.
Because other people are so important to our lives, it would make sense for our perceptual and cognitive systems to be specifically attuned to other humans, their appearance, and the sounds they make. It appears that many social species have anatomical and neural structures devoted to the task of identifying conspecifics (that is, members of the same species) and gathering relevant information about them (e.g., Romanski, 2009). If music is able to activate human-detecting neural pathways in our brains, this could provide a partial explanation for why music can be so bewitching.
While mimetic theories of music have existed from antiquity, only a subset have explicitly proposed that music mimics human beings. Instead, several other subjects have commonly been suggested. The Pythagoreans felt that music instantiates musica universalis, and compels the soul to resonate sympathetically with divine harmonies. For Charles Batteaux, eighteenth-century French philosopher and aesthetician, music serves as a ‘portrait of the passions,’ imitating Nature’s beauty as all beaux arts do (Neubauer, 1986, p. 61). Batteaux’s fellow French académicien Jean-Baptiste Dubos believed that music imitates ‘all those sounds with which nature herself expresses her sentiments’ (ibid. p. 63). A century later, German philosopher Arthur Schopenhauer claimed that music represents ‘the will itself with nothing intervening.’ (Dahlhaus, 1982, p. 42). The field of possible referents seems limitless.
Nonetheless, the view that instrumental music mimics the human voice has also been prevalent since antiquity. Several, including Plato and Galileo, have argued the inferiority of instrumental music to vocal music from precisely this premise. Still others have pointed out resemblances to human features other than the voice. For example, Enlightenment lawyer and music theorist Roger North wrote:
[M]usick is a true pantomime, or resemblance of humanity in all its states, motions, passions, and affections. And in every musicall attempt reasonably designed, humane nature is the subject, and so penetrant that thoughts, such as mankind occasionally have, and even speech it self, share in the resemblance so that an hearer shall put himself into the like condition, as if the state represented were his owne.
(Musicall Recollections III: f.48v, cited in North, 1728/1990, p. 46)
North’s stance on musical anthropomimesis can be viewed as a direct precursor of the present perspective.
An argument that a particular type of sensation is at some level perceived as being human could be supported by several types of evidence. First, a distinct mode of perception specialized for other humans ought to be automatic and mandatory, possibly producing a strong and distinct phenomenology. Second, presuming it is more costly to mistake a human for something non-human than the reverse, one would expect to find several instances where non-human percepts are perceived as human. Third, these faculties ought to appear very early in life, because perceiving-as-human would enable infants to know which sensations to learn from. Fourth, there ought to be identifiable neural pathways that support such percepts, whether they are completely innate or acquired from experience. Finally, if the ability to perceive something as human is a special, modularized capacity, then one might expect to find specific deficits in this ability.


Facial Perceiving-as-Human
An excellent example of an everyday ‘perceiving-as-human’ experience can be found when one gazes at another person’s face. Faces are of primary importance in our social world; we use them not only to recognize the identities of others, but also their intentional and affective states. Moreover, it appears that facial perception might be automatic and mandatory, producing a particular phenomenological quale (Palermo & Rhodes, 2007). The strength of this committed face perception apparatus is demonstrated by the human penchant to see faces in many places other than on other people, as the two images in Figure 1 make vivid.
The image on the left depicts a rock formation identified by the Viking 1 spacecraft when photographing Martian Cydonia in 1976. This mountain in particular bears a striking likeness to a human visage. On the right is a more commonly-encountered ‘face’: an electrical outlet. Although either image has only a coarse, minimal resemblance to an actual human face, both images are nonetheless strongly suggestive, creating an irresistible compulsion to see eyes and a mouth. The mind’s hair-trigger for face identification also leads us to commonly imagine faces in clouds, the moon, and the front of some automobiles. This tendency to incorrectly find meaningful content in inappropriate places has been called pareidolia, literally, ‘wrong image.’
It is clear that despite the spuriousness of such pareidolic percepts, things ‘perceived-as-human’ can nonetheless be quite compelling. A plausible explanation for this phenomenon would be that certain low-level features of face-like images—such as eye-like and mouth-like shapes in an upright orientation—automatically activate our face-processing neural machinery, a view supported by recent neurological evidence (Hadjikhani et al., 2009). Face processing has been linked to specific cortical tissue in the fusiform gyrus (Sergent et al., 1992; Kanwisher et al., 1997) as well as a subcortical pathway involving the superior colliculus, pulvinar and amygdala (Johnson, 2005). Rapid, spontaneous activation of these pathways in response to face-like stimuli could explain why facial perception seems to be so automatic, rapid, and irresistible.1 Even neonates with an average age of 36 hours have the capacity to recognize faces and mimic the facial expressions they see (Field et al., 1982).
The existence of a special facial perception faculty is also suggested by pathological deficits in face discrimination, recognition, and perception, together referred to as prosopagnosia, or ‘face-blindness.’ Although otherwise unaffected, people with acute or congenital prosopagnosia are often unable to recognize the faces of friends, family, or even themselves. Because this deficiency is specific to faces, it indicates there might be some modular capacity underlying facial perception that could be individually disabled.
Notably for the present study of musical anthropomimesis, biological tendencies of the human perceptual system are also ripe for artistic exploitation, as is shown by several works of trompe l’œil art. C. Allan Gilbert’s famous illustration All is Vanity, shown in Figure 2, deliberately manipulates the human propensity to see faces in minimal stimuli. The anthropomimetic characteristics of pareidolic faces can also trigger perception of emotional or affective states. As Davies (2010) has pointed out, when a visual percept has features that resemble a human emotional expression, we might perceive it as expressing an emotional state. It seems likely that musical art could produce its compelling expressivity in similar ways.

Three Forms of Musical Anthropomimesis
Music resembles at least three types of human-produced sounds, each of which might activate specialized human-perceiving neural pathways. First, music makes use of pitched tones that resemble (or are in fact produced by) the human voice, corresponding to a communicative animacy cue. Second, musical beats evoke imagery of human ambulation, corresponding to a locomotive animacy cue. Finally, pattern-based aspects of musical construction indicate an intelligent agent might have created the signal. In all, music’s trifold similarity to voice, gait, and language could potentially activate three separate perceiving-as-human systems. If so, this would explain its ability to capture our attention, as well as its capacity to express affective, intentional, and emotional states so strongly.
The view that music mimics humans ought to be clarified in light of the many other things music can imitate. Musicians and composers have often availed themselves of music’s ability to imitate any number of natural sounds, settings, or topics, from Josquin’s “El Grillo” to Edvard Grieg’s “Morgenstemning” or Leroy Anderson’s “Sleigh Ride.” This fact of artistic freedom is completely compatible with the idea that low-level processing of perceived sounds might yet follow preordained paths. Certain perceptual machinery may always treat music at some level as though it came from a human source, whether the composer used musical word-painting or not.
A final caveat should be mentioned regarding the scientific research that will be cited. The field of neuroscience is young and moves quickly; current neuroscientific studies are often limited to identifying possible biological underpinnings of long-held assumptions, ancient theories, or more recent psychological results. While the precise neurological evidence cited here might later be superseded, the salient point is the plausibility of such mechanisms, if not their detailed structure.
Notes and Voice
The idea that music shares close kinship with the human voice is anything but obscure: the voice has retained an important place in music throughout western history. Plainchant and Medieval polyphony are thought to have been performed completely without instrumental accompaniment, a practice that gives rise to the musical meaning of a cappella (Leech-Wilkinson, 2002). Writers from the Enchiriadis author (c. 850) to Leonard Bernstein (1976) have invoked linguistic comparisons with music, with countless authors suggesting that language and music share a common origin (e.g., Rousseau, 1782). To better understand relationships between music and the voice, it will be necessary to consider how musical and vocal sounds stand out from other ecological noises.
From a biological perspective, the sound of a human voice can be understood as just one instance of vocal communication sounds in general. A great many species signal one another using pitched tones against a backdrop of unpredictably random acoustic noise. Signalling apparatus such as vocal folds or syrinxes are able to produce sounds with energy concentrated at just a few frequencies, making pitched tones audible at longer distances than the same amount of sound energy would be if spread out over the sonic spectrum. This basic principle of vocal communication could be seen as what Dennett (1995) might call a Good Trick: an excellent evolutionary solution to a problem that would be expected to arise again and again.2
To humans, voices are indeed quite special sounds. A human voice, whether speaking, laughing, wailing, or humming, potentially carries as much information as does a human face (Belin et al., 2004). We recognize our family members and best friends merely by the sound of their voices, and can also tell if they are excited, bored, sarcastic, or frightened. We can quickly identify the sex and approximate age of people simply by hearing them on the phone, and we can even make a guess as to what part of the world they come from. Because of its distinctive character and informational richness, a human voice, much like a face, might be expected to evoke a particular mode of perceiving-as-human.
As previously suggested, certain sounds—such as factory whistles or alarms—might be perceived as being voicelike if they carry pitch or undulate like a voice could. This similarity is precisely why sirens are said to wail, engines to roar, and wheels to squeal. If metaphors such as these are in fact Lakovian cognitive metaphors rather than mere linguistic ones, they might reflect underlying perceptual predispositions. All sounds that are perceptually similar enough to pitched vocal sounds could be processed to some extent as though they were vocal sounds. The subset of these sounds that specifically resembles the timbre and pitch range of the human voice could move beyond mere perceptual animacy and instead extend to perceptually-relevant anthropomimesis.
Just as our hypersensitivity to face-like percepts can lead us to see faces where they do not exist, hypersensitive voice identification processes can result in hearing pareidolic voices. The auditory equivalent of a face on Mars or in an electrical socket might be something like hearing pained groans in the radiator system, or perhaps hearing an alto saxophone as a weeping widow. It is easy to imagine how blowing wind could be heard as a voice as well, whether at a seance or a campfire. Auditory pareidolias have even fueled occult movements: some twentieth century spiritualists have claimed to hear voices in radio static, tape noise, or other mechanical sources, believing them to be paranormal voices from the deceased or divine (Banks, 2001).
There appear to be particular regions of the primate and human brain specifically attuned to conspecific vocalizations (Belin et al., 2000; Fecteau et al., 2004; Petkov et al., 2008; Romanski, 2009), as well as areas devoted to recognizing vocalizations in general (Lewis et al., 2005). Similar to prosopagnosia, cases of phonagnosia—problems with voice recognition and discrimination—occur in both acute and congenital forms (Van Lancker & Canter, 1982; Garrido et al., 2009). Adding to the evidence that voice perception is a specialized faculty, it appears that infants selectively attend to voices at a very young age (Vouloumanos & Werker, 2007).
Hearing Voices in Musical Lines
For facial perception, it seems that two rudimentary eyes and a mouth, oriented properly, are sufficient to trigger a specific face perception mode. What might the analogous perceptual features be that indicate something should be perceived as a voice?
Several psychophysical studies have investigated the sound features that listeners use to classify sounds, such as harmonicity, spectral shape, frequency, and amplitude envelope (see, e.g., Kidd & Watson, 1987; Christensen & Humes, 1996). A recent study by Gygi et al. (2007) asked four participants to make 10,000 pairwise similarity ratings for a collection of short sounds. A multi-dimensional scaling technique was then used to determine which three composite factors could best explain the similarity of the sounds. The first, most important dimension corresponded to the sound’s harmonicity, with animal sounds, speech, laughter, and musical instruments clustered together on one end of the dimension, and inharmonic noises such as a typewriter, drums, footsteps, or hammering on the other.
Because vocalizations are distinguished from other environmental sounds by the presence of harmonic overtones—concentrated energy at particular frequencies—the harmonicity of sounds might be a good indicator that they are vocalizations. Assuming that conspecific vocalizations are particularly special sounds, it would make sense that the human hair-trigger for voice perception might be wired to harmonicity detectors.
Neuroimaging studies have provided additional evidence that musical instruments and the voice are cortically processed in similar ways by merit of their high degree of harmonicity. It has been proposed that vocal sounds are processed along a cortical pathway in which acoustic features such as harmonicity are used to route the signal toward increasingly specialized processing locations (Lewis et al., 2009; Talkington et al., 2012). At lower levels of processing, musical instruments and voices would presumably be processed identically. Consistent with this view, at least one phonagnostic has exhibited impaired ability to recognize musical instruments as well as voices (Hailstone et al., 2010).
In a representative neuroimaging study, Leaver & Rauschecker (2010) employed functional magnetic resonance imaging techniques to measure cortical activation when hearing different sounds. Participants heard recordings of human speech sounds (isolated phonemes), musical instruments, songbirds, and other animals. Of these four, both human voices and musical instruments evoked responses strongly in the same region of the anteroventral auditory cortex, consistent with the view that their processing overlaps. Interestingly, Leaver & Rauschecker’s musical instrument recordings exhibited a slightly higher harmonics-to-noise ratio than speech and a much higher pitch strength. If the hypothesis that harmonicity is an important identifying perceptual marker for speech is correct, then perhaps musical instruments could be viewed as a distillation of this salient feature of the voice.
In addition to harmonicity, there are other similarities between human voices and instrumental music that distinguish them from animal sounds. Both utilize the same approximate pitch range and clef-based notation, the standard form of which possibly arose from vocal ranges. Moreover, both speech and musical melodies exhibit similar interval sizes, with smaller intervals generally favored and intervals a fifth or larger being relatively rare (Patel, 2008, p. 221; Huron, 2006, p. 74; Vos & Troost, 1989). Even though several instruments can transcend the pitch and speed-based constraints of the voice, it seems anecdotally that the most memorable melodies are those that can be sung. It is to this idea that we now turn.
Motor Theories of Speech and Music
When considering the evolution of vocal communication, it is clear that any sound meant to be heard would be completely unhelpful if it could not be perceived. This could be viewed as a basic problem of any communication system, which must rely on the signaller and receiver using the same ‘code.’ The faculties of vocal production and vocal perception ought therefore to evolve concurrently and congruently, including the musculoskeletal and neural machinery for both.
While the neural substrates for voice production and perception could theoretically coevolve as two separate systems, it might be more efficient and parsimonious for the two to overlap. In other words, the perceptual process might be expected to rely in part on the premotor and motor neurons responsible for the production of vocal sounds, engaging them in an ‘off-line’ mode during perception. This ‘simulationist’ account is the essence of the ‘motor theory’ of speech perception proposed by Haskins Laboratory researchers in the 1950s (see Liberman et al., 1967; Liberman & Mattingly, 1985). Because speech sounds are so complex and vary so much from speaker to speaker, Liberman and his colleagues proposed that it is not phonemes per se that are perceived, but rather anatomical configuration of the vocal apparatus. This would account for how listeners are able to perfectly understand speech from a broad range of speakers, even though the constituent sounds themselves might vary dramatically.
The motor theory of speech perception has been bolstered by experimental evidence collected using direct neuronal measurements. Studies with nonhuman animals have revealed that the perception and production of vocal sounds can activate identical neurons. For example, several species of birds exhibit activation of motor nerves when perceiving birdsong (e.g., Williams & Nottebohm, 1985). Evidence for a broader simulationist theory of behavior perception has also been observed in nonhuman primates. Certain neurons in the monkey premotor cortex have been identified which respond both to actions performed and perceived, across both visual and auditory modalities (di Pellegrino et al., 1992; Gallese et al., 1996; Kohler et al., 2002). The existence of these so-called ‘mirror neurons’ suggests that simulationist hypotheses of perception might extend quite broadly (Galantucci et al., 2006).
It has been suggested that a motor theory of perception might have considerable explanatory power for music as well (Nussbaum, 2007; Zatorre et al., 2007). For those who would suggest that music is able to ‘resonate’ with us, or that it can induce affective states through an empathic sense, mirror neurons might provide a reasonable anatomical substrate. If this is the case, then when we hear musical lines, we hear voice-like stimuli that not only draw our attention, but activate the same neural mechanisms that we use to produce musical sounds ourselves.
Beats and Gait
In addition to vocal mimicry, music exhibits a strong resemblance to the human rhythms of walking. A great deal of music worldwide is arranged according to an underlying pulse, and moving to music appears to be a cross-cultural universal (Brown, 2003). Not only do compositions tend to be written at tempi close to a typical walking tempo of 120 beats per minute (Murray et al., 1964; Fraisse, 1982; Moelants, 2002), this tempo also appears to be the easiest to synchronize one’s paces with (Styns et al., 2007), and is approximately the optimal range for musical beat perception (Fraisse, 1982). The many parallels between biological motion and musical meter have led Van Noorden & Moelants (1999) to propose a ‘resonance theory of tempo perception’ that incorporates both driving energy and dampening factors. Experimental evidence has even linked the characteristic tempo changes of final ritardandi with the velocity of runners coming to a stop (Friberg & Sundberg, 1999). It is worth considering whether rhythmically metered music is naturally perceived not only in terms of auditory constraints at the extremes, but in terms of physiological optima in the center.
Much like the face and voice, a person’s gait provides a great deal of information about them, including their identity, affective state, and intentions. The sound of walking is easily distinguished from sprinting or limping, and the sound of speeding up is quite different from the sound of slowing down. A toddler has a considerably different gait from his grandmother, and the two would almost certainly be aurally distinguishable. Even a person’s sex can be determined solely by the sound of their footsteps (Li et al., 1991). Because of the information these sounds potentially carry, one might expect gait-like percepts to follow specialized processing pathways that extract relevant information about the walker’s behavior, mood, or identity.
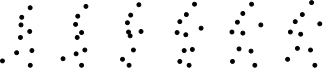
In the visual domain, there is abundant evidence that human gait is readily perceived with only minimal cues. Moving displays of a few strategically-placed dots are sufficient to suggest motion characteristic of human gait (Johansson, 1973). Figure 3 depicts a point-light display of the type used by Swedish psychologist Gunnar Johansson, who demonstrated that biological motion could be perceived with no information about the form of the walker’s body or limbs themselves. Not only is this impression uncanny and irresistible when observed, the capacity to perceive biological motion from moving dots appears even in two-day old newborns, who attend more to upright biological motion displays than their inverted counterparts (Simion et al., 2007). Analogously to prosopagnosia and phonagnosia, pathological deficits in biological motion perception also appear in some people, such as schizophrenics (Kim et al., 2005) and autists (Blake et al., 2003; Parron et al., 2008).3 In all, it would seem that the visual perception of locomoting animals and humans could rely on specialized systems, whether fully innate or acquired through experience.
The auditory perception of biological motion is somewhat less studied than visual perception, but scholarly literature regarding musical beat perception does exhibit several parallels to that of faces, voices, and biological motion. The perception of regular beats seems to quickly recruit perceptual pathways that predict their continued occurrence; disruption of regular rhythms can elicit characteristic preconscious brain wave responses (see Naatanen, 1995, for a review). Additionally, infant studies have suggested that the ability to perceive beat and meter appears at a very early age (Phillips-Silver & Trainor, 2005; 2007). Specific deficiencies in the auditory perception of beat and meter have also been identified. At least one person with congenital amusia has been diagnosed with musical ‘beat deafness,’ without exhibiting other musical deficits (Phillips-Silver et al., 2011), suggesting a discrete contribution of beat-processing pathways to musical enjoyment.
Recalling the motor theory of vocal perception, visual perception of biological motion and auditory perception of beat both appear to make use of premotor cortical regions. Biological motion in point-light displays reliably activates parts of the premotor cortex, consistent with a simulationist theory of ambulation perception (Saygin et al., 2004, 2007). Theorizing along these lines, psychologist Neil P. M. Todd (1999) proposed an explicit role for motor pathways in the perception of musical rhythm, and more recent studies have revealed that the perception of musical beat does in fact activate the premotor cortex as well (Grahn & Brett, 2007). If musical beat is processed by the same neural architecture that underlies ambulation, then this could provide some explanation for our tendency to spontaneously entrain to music, synchronizing our movements with the beat by tapping, nodding, rocking, or dancing. In both the visual and auditory senses, it seems that locomotion can result in a simulationist mode of perceiving-as-human.
Evidence from medical science has also suggested surprising links between beat perception and ambulation. A striato-thalamo-cortical network in the brain has been proposed to mediate beat perception, linking the premotor cortex with the basal ganglia, which are thought to mediate purposeful movement and timing tasks (Zatorre et al., 2007; Grahn & Rowe, 2009; McAuley, 2012). When the basal ganglia are compromised in patients with Parkinson’s disease, deficits arise in controlling and pacing muscle movements, resulting in these patients’ characteristic Parkinsonian gait. In addition to problems with movement and walking, patients with Parkinson’s disease have problems perceiving musical beats and performing timing tasks (Artieda et al., 1992; Elsinger et al., 2003; Grahn & Brett, 2009). In fact, it seems that deficiencies in timekeeping might lie at the root of walking difficulties in Parkinson’s patients: providing somebody with Parkinson’s with an external beat to synchronize with can cause dramatic improvements in his gait (McIntosh et al., 1997).
Musical relationships with motion need not stop at the beat produced by walking, and many theorists have related musical rhythm to kinematics more broadly (see Repp, 1993; Todd, 1992, 1995). When MacDougall & Moore (2005) used accelerometers to record the daily motion of several study participants, several oscillation frequencies in whole-number ratios were detectable in various body parts, such as the hip, head, or ankle. There is also some evidence that individual differences in body morphology might contribute to preferred musical tempi (Todd et al., 2007; Utley, 2009; Grahn & McAuley, 2009). Although relationships between beat processing and walking have not been entirely worked out, it would seem that close ties between beat and body motion could provide a low-level biological basis for the infectious quality of musical beat.
Finally, it is worth considering that without the ability to move one’s body, there would be very little reason for an advanced timing faculty to evolve in the first place. Organisms without articulated musculature (such as plants) seem not to have any advanced sense of time, instead relying on various environmental cues to regulate their growth patterns. It was previously suggested that a motor theory of vocalization would be evolutionarily parsimonious, because both the productive and perceptual capacity could share the same neural substrate. The same argument could be made for locomotion and metric timekeeping.
Patterns and Language
In addition to having voice-like and gait-like characteristics, musical lines are language-like in that they exhibit syntactically arranged patterns of notes and rhythms. Any sight or sound that appears to have repeated subunits might suggest that some energy source put them in order. Whether or not these units actually convey information, complex patterns and embedded regularities could indicate that an intelligent creature lies behind the percept. Therefore, sounds that seem to contain embedded information, such as spoken language, morse code, or radar blips, might be expected to encourage more careful listening than comparatively less organized sounds, such as chuckles, grunts, or undulating sirens. Music, with its tendency to exhibit hierarchical organization and repeating subunits, certainly gives the impression of being syntactically arranged, and it very often is.
Would it be reasonable to postulate a specific ‘mode of perception’ for pattern recognition? It would surely seem that humans are adept at recognizing patterns, from points of light in the night sky to tesselations of brickwork. Chess grandmasters can identify complex board positions they have encountered before, and even make intuitive judgments regarding ones that they have not. There is even evidence that people can implicitly learn organizational patterns behind temporal sequences of visual and auditory stimuli, even without being consciously aware of what they are learning (Reber, 1967). For instance, both infants and adults appear able to implicitly learn novel grammars of pitched tone sequences (Saffran et al., 1999). But by far the most striking instance of human pattern perception is language. Extracting meaningful information from patterns of printed and spoken words is a monumental feat, surpassed only by a child’s ability to acquire this capacity without explicit instruction.
On the surface, the processing of linguistic patterns resembles other types of perceiving-as-human, in that specialized neural machinery seems to underlie the process. Without delving too deeply into debates over the domain-specificity of the linguistic capacity, there can be no doubt that at least two language processing centers, Broca’s and Wernicke’s areas, exist on the human cortex. The ability to recognize linguistic patterns also appears very early in life, with infants even preferring the rhythmic cadence of their mother’s language over that of other tongues. Well-described linguistic deficits, or aphasias, have also been linked to lesions in Broca’s or Wernicke’s areas, suggesting some modularity of the ability to understand and produce language.
Similarly to the modes of perception already discussed, it appears that there are several examples where humans are prone to hyperactive pattern recognition (see Foster & Kokko, 2009). This mistaken discovery of patterns in random or meaningless data has been called apophenia, sometimes manifesting as conspiracy theories or superstitions, and other times as the simple perceptual recognition of spurious visual or auditory patterns. For example, a fast-spreading rumor that British rock musician Paul McCartney had died grew rapidly in 1969 after ‘hidden reversed messages’ on a Beatles recording were heard (Reeve, 1994). In the coming decade, fundamentalist Christians soon began to complain about Satanic messages that were audible in reversed popular records, such as Led Zeppelin’s 1971 rock anthem “Stairway to Heaven” or Styx’s 1981 release “Snowblind” (Smith, 2011). In each of these examples, a voice-like sound was certainly present, but patterns of speech that were absent (i.e., English words) were mistakenly identified. These incorrectly heard backward messages could be described as instances of auditory apophenia, and ones that involved anthropomimetic hallucinations at that.
Because musical sounds tend to exhibit deliberate syntactic organization, it seems possible that the built-in pattern detectors normally applied to language or recognizing other structured events might also be engaged while listening to music. In fact, there is considerable evidence that music and speech processing share overlapping cognitive resources, which lends credence to a resource-sharing hypothesis of language and music (Patel, 2003). Both musical and linguistic signals can evoke similar event-related brain potentials (Besson & Faïta, 1995; Patel et al., 1998), and the processing of musical syntax appears to make use of linguistic areas in the brain (Patel, 2008, p. 276). To the extent that languages are perceived as coming from human sources, it would seem that syntactic music would be too.
Could the processing of spoken syntax and patterns of musical tones really be mediated by the same neural pathways? After all, most western languages utilize words composed of vowels and consonants as their syntactic elements, not musical notes. However, this apparent separation between language and tone is not a cultural universal—in fact, the majority of the world’s languages are tone languages, with some exhibiting up to five discrete level tones (Patel, 2008; Fromkin, 1978). In tone languages, linguistic syntax explicitly depends on the sequences of tones being used, highlighting the connection between musical and lexical syntax. Instruments such as drums, whistles, or stringed instruments can even serve as ‘speech surrogates’ by speakers of tonal languages. Games can be played based on guessing the linguistic message communicated on a guitar or drum, and important messages can even be whistled across long distances (Patel, 2008, p. 48). The existence of such speech surrogates provides direct evidence that some musical instrumental sounds can be readily ‘perceived as human.’
In addition to syntactic orderings of pitch, it is possible that some rhythmic regularities in music are processed by the same brain regions responsible for linguistic rhythm. Iversen et al. (2008) reports that Japanese and American listeners tend to group identical rhythmic stimuli differently, in ways reflective of their native languages’ characteristics. There is also neurological evidence that similar regions of the brain are involved in processing both musical and linguistic phrase boundaries (Steinhauer et al., 1999; Knosche et al., 2005). Interestingly, tapping musical polyrhythms seems to activate linguistic areas of the brain (Vuust et al., 2011), suggesting that some forms of musical rhythmic complexity are closely related to language processing.
Musical lines therefore could be said not only to mimic human noises by having the harmonicity and contour of vocal sounds (as laughs, cries, grunts, wails, or screams do), but also because they use tonal and rhythmic units syntactically, resulting in a distinct mode of musical perception and enjoyment (see, e.g., Meyer, 1956; Cooke, 1959; Lerdahl & Jackendoff, 1983; Narmour, 1990; Huron, 2006). Because musical lines make use of patterns—even if they do not map directly onto any known language, they still might suggest an intelligent human being produced them.
Conclusion
This chapter has argued that music is compelling in part because of the anthropomimetic character of notes, beats, and patterns, which in turn reflect three aspects of human-created sounds: voice, gait, and language. These modes of perceiving-as-human could underlie music’s capacity not only to be perceived as emotional or intentional, but also its ability to capture our attention so strongly. A melodic line resembles a voice by merit of being pitched, can resemble gait by being metric, and can contain information by having motivic patterns of rhythm and pitch.
Ethnomusicologists and anthropologists have long observed that music plays an integral role in human cultures, with singing, dancing, and group participation being crucial aspects. To western musicians and nonmusicians alike, it’s enjoyable to sing along or move along with music—consistent with the idea that music perceived-as-human tends to be processed using the same premotor pathways that would be used to create the sounds.
That not all western art music is meant for singing or dancing appears to be somewhat unusual among musical cultures. It would be interesting to know the degree to which our perceptual capacity constrains western art music to remain within the realm of sounds that could be produced by the body itself. If motor theories of musical processing are correct, then even a person with no prior biases might still be unlikely to enjoy music incompatible with their physiological and psychological dispositions, even if the music falls within the extremes of their perceptual limits.
If musical lines are perceived in terms of their anthropomimetic character, this leads naturally to some predictions about how music might express certain types of emotion. For example, polyphonic instrumental music with many musical parts might imply a social situation with many participants, whereas instrumental music with only a single musical line would imply only a limited number of participants. The next chapter will describe three psychological experiments regarding the perception of multiple polyphonic voices and perceived musical emotion.
Footnotes
Some parts of the ‘fusiform face area’ have been observed to activate in response to other objects as well (Grill-Spector et al., 2006), suggesting the region might represent more generalized ‘expertise.’ This would not conflict with the idea that facial perception recruits specialized pathways. ↩
Sure enough, in the context of radio broadcast, humans have reinvented the same conceptual solution. ↩
Interestingly, both autism and schizophrenia are also associated with deficits in the perception of vocal prosody, or ‘speech melody.’ ↩